I study RNA quality control in aging yeast, combining individual cell histories, molecular measurements of age-enriched populations and human-reviewed image analysis.
A changing nuclear boundary. A consequence for the genome.
Question. How does nuclear-pore remodeling contribute to chromosome loss in aging yeast?
Result. Our 2025 study linked nuclear-basket displacement to pre-mRNA leakage and chromosome loss. Removing introns from three chromosome-segregation genes suppressed the chromosome-loss phenotype.
Why it matters. A structural change at the nuclear pore is connected to an intron-dependent failure of cell function.
My contribution: formal analysis, validation and experimental investigation, plus manuscript review and editing.
Published contribution statement
Formal analysis, validation, investigation, and writing – review and editing, as recorded in the published author-contribution statement. This was a collaborative study; the full author list appears above.
DOI: 10.7554/eLife.104530.3
Have a complementary question, assay or set of strains? Let’s explore a focused research collaboration.
A cell is more than its genes. It matters how it handles their messages.
My current PhD research asks how nuclear RNA quality control changes during aging and stress. A mother yeast cell produces successive daughters; the number produced over its lifetime is its replicative lifespan.
New to RNA biology? Start here.
RNA carries genetic instructions from DNA toward the machinery that makes proteins. Many newly made RNA messages contain segments called introns, which are normally removed by a process called splicing. Cells also control which messages can leave the nucleus.
I study how this processing and quality control change with age. The immediate aim is to understand mechanisms of aging in budding yeast. Whether a finding applies to human aging is a separate experimental question.
Explore my current research questions
I.
Which RNAs are allowed to leave?
How are incompletely processed transcripts retained in the nucleus, and what allows them to escape? The distinction between processing an RNA and controlling its export is central to the question.
RNA surveillance / Nuclear retentionII.
What changes at the nuclear pore?
The nuclear pore connects the nucleus with the rest of the cell. I study how changes in this architecture relate to RNA quality control as a cell grows older.
Nuclear architecture / AgingIII.
When does a molecular change affect the cell?
A molecular change is not yet an explanation. The aim is to distinguish correlation from cause, and connect altered RNA handling to a measurable consequence for the cell.
Mechanism / Single-cell biology
03 How I do the work
Two views of the same problem. A cell’s life. Its molecular state.
One approach follows the life of an individual cell. The other collects aging cells in sufficient numbers to measure their molecules. Together, they let us study aging at two different scales.
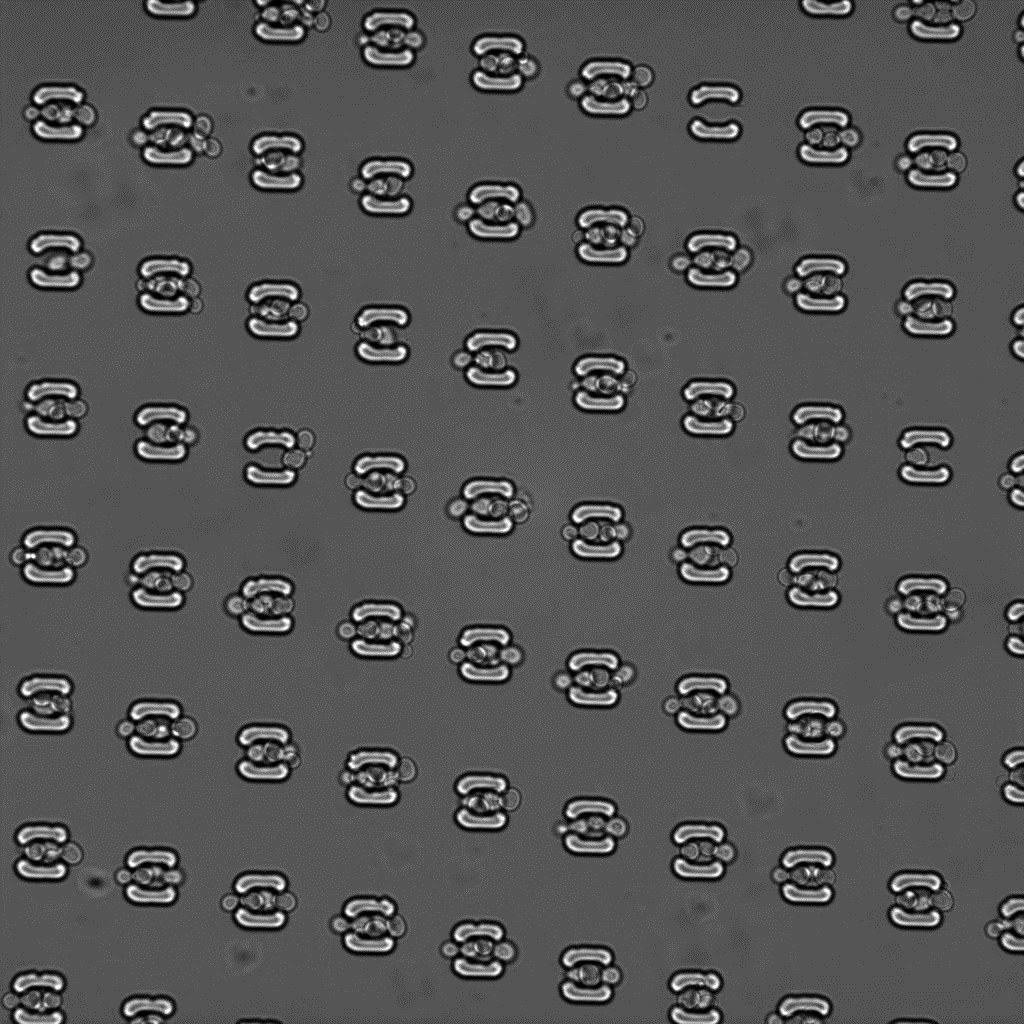
Microscopy inside an aging chip. The curved structures hold yeast cells in place so they can be followed over time.
The life of one cell
Watch a cell grow old.
Question
When does a cell’s behavior change during its replicative life?
Approach
Microfluidic traps and repeated imaging follow individual yeast mothers as they produce daughters.
Readout
Division histories and replicative lifespan; fluorescence trajectories where a suitable reporter is used.
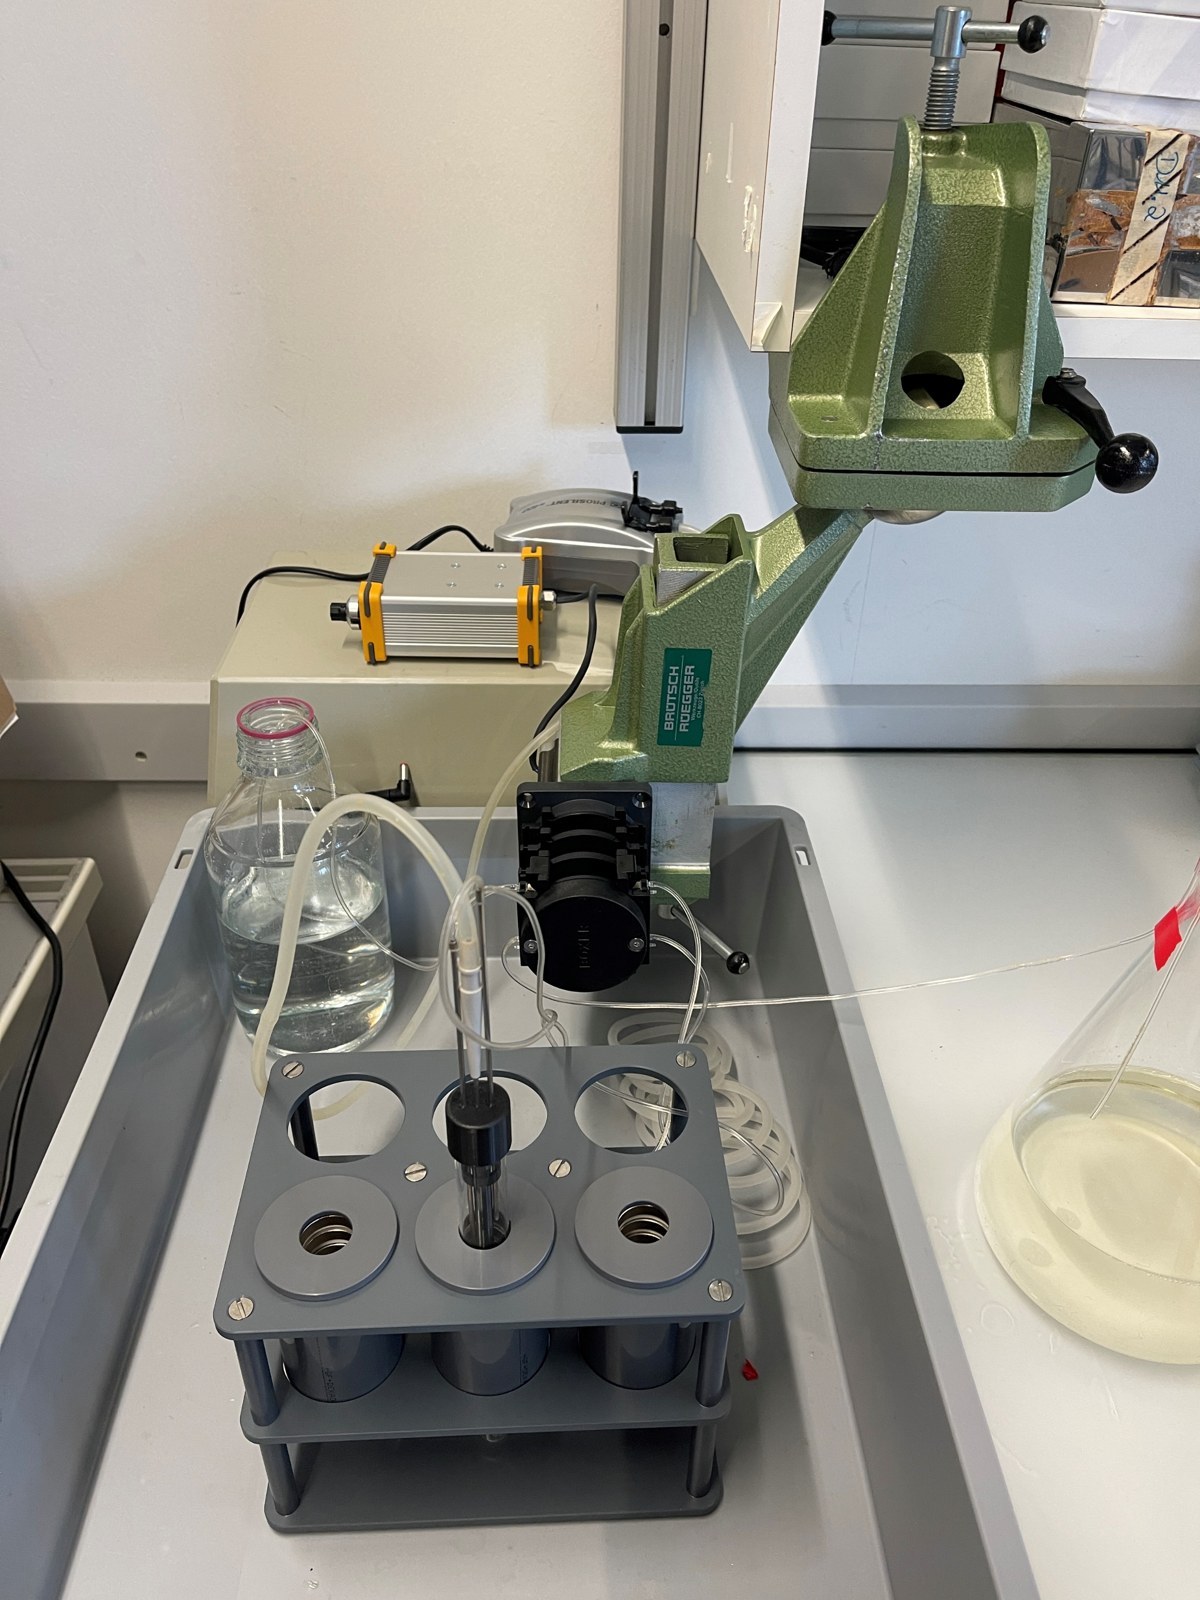
MAD bioreactor setup in the Barral laboratory. The tube, magnetic rack and pumps allow aging mother cells to be retained in flowing culture.
The molecules of a population
Collect aging cells. Measure what changes.
Question
Which molecular features differ between younger and age-enriched yeast populations?
Approach
The Miniature-chemostat Aging Device (MAD) retains magnetically labelled mothers while daughters wash out.
Readout
Age-enriched populations for RNA and other molecular measurements, rather than perfectly age-pure samples.
These approaches address complementary scales: the bulk samples are not the same cells followed in the movies.
From movies to reviewed cell histories.
I develop image-analysis workflows to organize trap-level images, support annotation, and extract division and lifespan summaries. Automated calls remain subject to human review; the workflow is still being developed and validated.
I learned the MAD approach with the Caudron laboratory in Montpellier and worked with the ETH workshop on our laboratory implementation. With thanks to Remo Zangger and Daniel Smith for the setup, and to Sung Sik Lee for the aging-chip platform. MAD was introduced by Hendrickson and colleagues, eLife (2018).
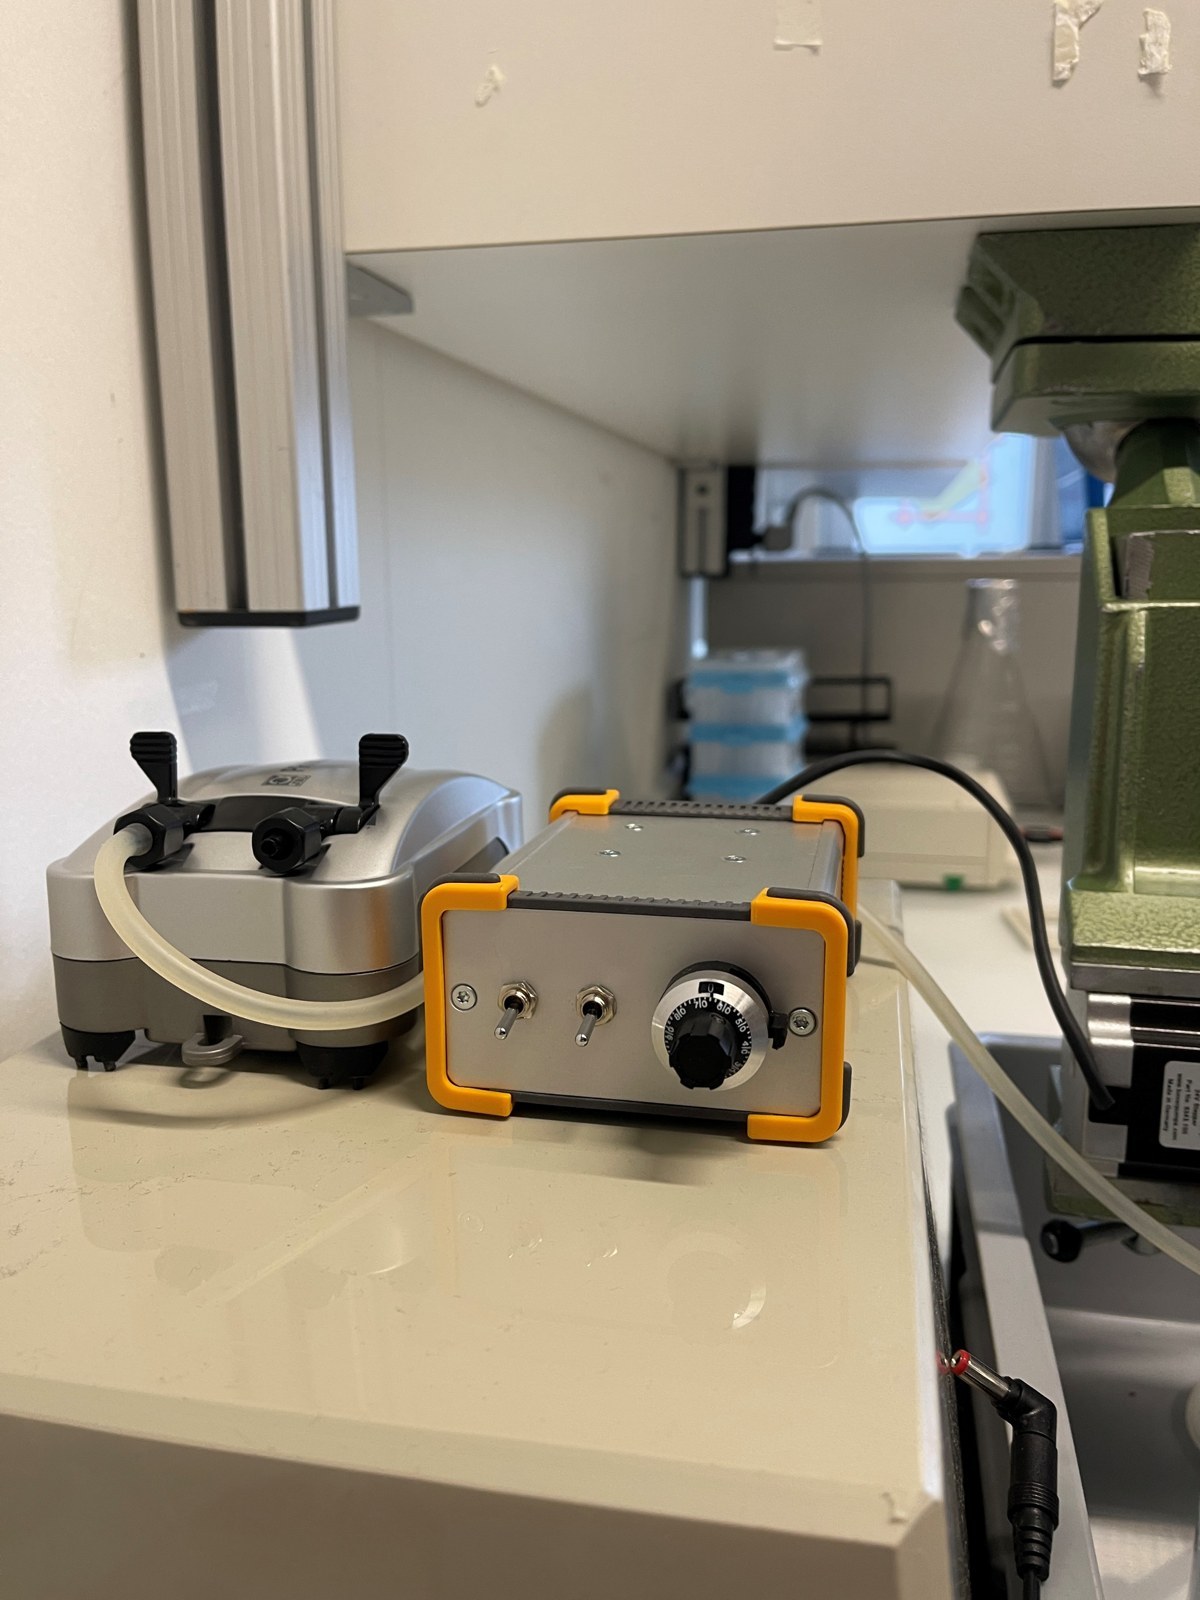
Inside the setup: pumps, controls and image sourcesPump and control equipment used in the MAD setup.
The microscopy frame and apparatus photographs are from slides 39, 48 and 49 of my 26 September 2025 lab presentation. The presentation date is not the acquisition date. These images illustrate the methods rather than a quantitative experimental comparison.
04 Working together
A focused question. A complementary collaboration.
I’m interested in research collaborations connecting cell histories with molecular measurements. A good fit brings a specific cellular-aging question and complementary strains, data, an assay, expertise or research resources.
First, a short research-fit discussion. We would agree a bounded question, each partner’s contribution, scope, resources and any laboratory access individually.
Does a yeast perturbation change when divisions slow or when a fluorescent reporter changes during replicative aging?
Could a molecular difference in your age-enriched yeast samples motivate a test in individual cell histories?
05 About
From Massachusetts to Zürich.
I trained at the University of Massachusetts Amherst and the Technion before joining the Barral laboratory at ETH Zürich. My work brings together biochemistry, genetics and cell biology to understand how RNA quality control changes as cells age.
Current
ETH Zürich
PhD researcher · Barral laboratory · Institute of Biochemistry